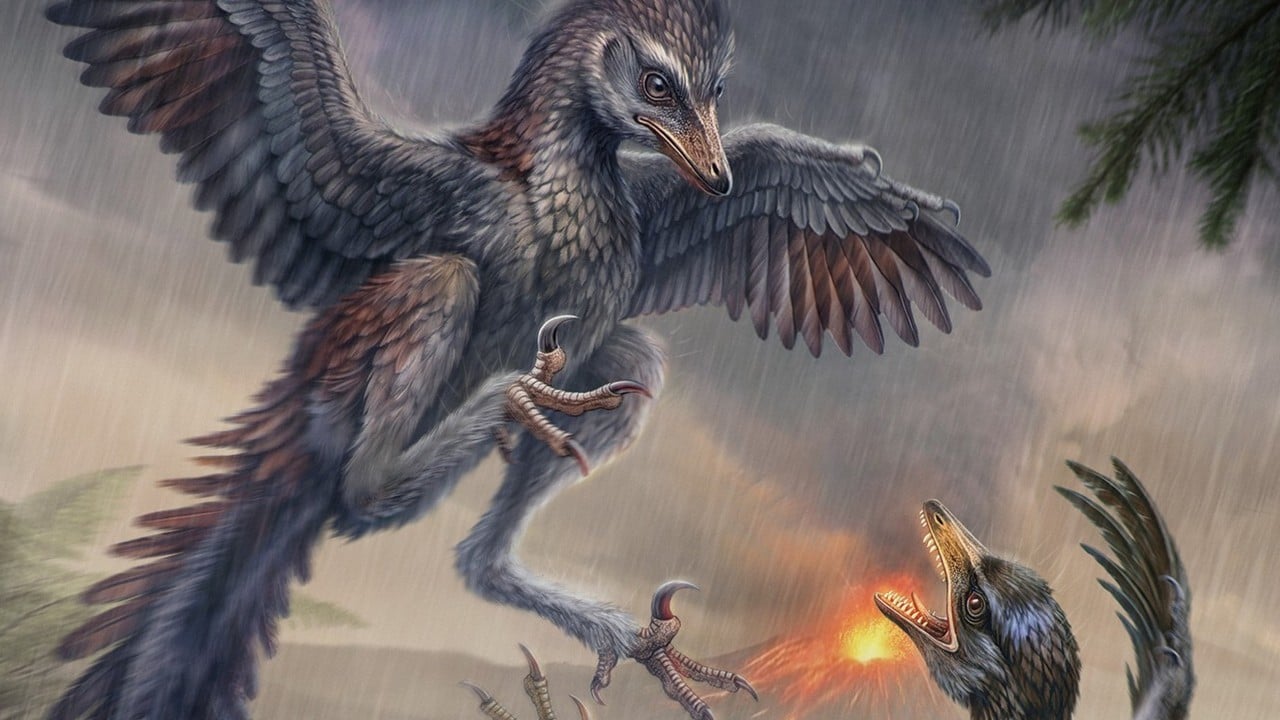
Popular science coverage routinely treats powered flight as the defining endpoint of early bird evolution, framing any flightless prehistoric avialan as an evolutionary dead end or an anomaly against Charles Darwin's descent with modification. That framing gets the causality backward. Flightlessness in early avialans was not a rejection of evolutionary progress; it was a recurring, energetically rational specialization driven by localized resource density, predator distribution, and developmental trade-offs across Mesozoic ecosystems. This analysis deconstructs the flawed narrative around flightless early birds, establishes a structural framework for evaluating flight loss in basal avialans, and maps the causal mechanisms that governed locomotion in the early avian clade.
To understand why sensationalized headlines misread Mesozoic fossils, we first have to separate observable anatomy from speculative storytelling. In paleontology, a known fact is a physical trait preserved in rock—such as fused carpometacarpals, shortened forelimb elements, reduced sternal keels, or dense bone cortex—alongside stratigraphic placement and phylogenetic position. An educated hypothesis is the functional or ecological explanation inferred from those traits, such as whether reduced wing proportions reflect terrestrial foraging, diving, or cursorial evasion. Confusing a fossilized bone with a complete behavioral biography is where popular articles stumble.
Deconstructing the Sensationalist Headline Trap
Headlines that pit a single fossil discovery against Darwin rely on a straw-man version of evolutionary theory. Natural selection does not optimize toward a universal ladder of complexity ending in aerial mastery; it filters heritable variation relative to local selection pressures and energetic budgets. When a fossilized early bird from northeastern China or elsewhere displays traits consistent with reduced or absent powered flight, the surprise belongs to modern expectations of linearity, not to evolutionary mechanics.
Sensational coverage typically makes three analytical errors when handling paleontological finds:
- Teleological framing: Treating aerial flight as a destination or superior state rather than one locomotor strategy among several competing for metabolic return.
- Single-trait reductionism: Inferring whole-organism ecology from a single bone proportion while ignoring limb ratios, pelvic geometry, and depositional environment.
- False novelty: Presenting a well-documented evolutionary pattern—repeated loss or restriction of flight across lineages—as an overturn of foundational biology.
A rigorous analytical approach strips away the drama and asks a sharper operational question: what ecological conditions made retaining full powered flight metabolically expensive or functionally suboptimal compared to alternative locomotor modes?
Known Facts Versus Educated Hypotheses in Early Avian Paleobiology
Rigorous analysis requires a hard boundary between empirical observation and interpretation. Taphonomy—the processes of decay, burial, and fossilization—selectively preserves certain tissues and environments over others. Fine-grained lacustrine sediments in regions like the Jehol Biota preserve delicate impressions of feathers and articulated skeletons at high resolution, yet soft-tissue organ systems, exact muscle fiber recruitment, and seasonal behavioral shifts rarely fossilize directly.
When researchers examine a basal avialan with reduced forelimbs or altered wing-loading ratios, the presence of specific skeletal dimensions is a fact. The exact speed at which the animal moved, the precise caloric savings of spending less energy on flight muscles, and the exact competitive trigger that favored ground or aquatic specialization are hypotheses tested through comparative anatomy, biomechanics, and phylogenetics. Treating hypotheses as settled facts weakens credibility; treating facts as mere guesses wastes hard evidence.
The Four Pillars of Early Avian Flight Loss
Rather than viewing flightlessness as an isolated oddity, we can model the emergence of flightless or flight-restricted early avialans across four interacting pillars. Each pillar represents a distinct set of constraints and payoffs operating on an organism over evolutionary time.
1. The Energetic Cost Function of Aerial Locomotion
Powered flight is metabolically demanding. Generating lift and thrust against gravity requires substantial pectoral muscle mass, specialized shoulder girdles, high-output cardiovascular and respiratory support, and structural reinforcement capable of handling aerodynamic loads without excessive weight penalties.
In evolutionary economics, every gram of tissue dedicated to flight apparatus carries an opportunity cost. If an avialan inhabits an environment where food, mates, and nesting sites are accessible on the ground or in shallow water without long-distance aerial transit, maintaining oversized flight musculature taxes the daily energy budget. Reducing reliance on powered flight reallocates metabolic resources toward growth, reproduction, or specialized foraging structures.
This creates a bottleneck for lineages operating on tight energy margins. When food resources are patchy and require traversing wide or hazardous terrain, flight remains a high-value mobility asset. When resources are concentrated locally and predation pressure is manageable without vertical escape, the return on investment for full flight capability drops.
2. Ecological Niche Saturation and Resource Partitioning
Evolutionary diversification accelerates when lineages partition resources rather than colliding head-on in identical niches. Early avialans did not appear in an empty sky; they radiated alongside pterosaurs, non-avian theropod dinosaurs, mammals, crocodyliforms, and diverse plant and insect communities.
Reducing aerial dependence opened alternative foraging zones. Consider two distinct ecological strategies in a wetland or forest-edge setting:
- Terrestrial and understory foraging: Exploiting leaf litter, burrows, or dense vegetation where broad wings create drag, snag on branches, or add unnecessary bulk during rapid ground maneuvering.
- Aquatic pursuit and surface foraging: Shifting limb mechanics toward paddling or diving, where buoyancy and hydrodynamic drag impose very different structural demands than airfoil lift.
A second limitation of purely aerial strategies appears in crowded canopy or brush environments. High maneuverability in tight spaces favors specific wing shapes and body plans, whereas ground-based or semi-aquatic niches reward different limb proportions altogether. Niche partitioning explains why flight capability is not a ratchet that only locks in one direction.
3. Predation Pressure and Escape Mechanics
Flight is widely assumed to be the ultimate escape mechanism, yet escape effectiveness depends on predator type, habitat structure, and life stage. Against fast aerial or arboreal predators in open spaces, taking wing offers clear advantages. Against ambush predators in dense cover, or when rapid burst movement on solid substrate or water is faster than launching into the air, alternative escape tactics can dominate.
Launching into flight from a standstill requires coordination, space, and time. If an animal can dart into dense cover, sprint across open ground, or submerge quickly, natural selection may favor ground or aquatic agility over long-range flight endurance. Predation acts as a selective filter on escape geometry, not a universal command to stay airborne.
4. Developmental Heterochrony and Life-History Trade-Offs
Evolutionary shifts in adult morphology frequently originate in changes to developmental timing, known as heterochrony. Accelerating, slowing, or truncating growth trajectories in specific skeletal elements can alter limb proportions without requiring wholesale reinvention of the body plan.
If selection favors earlier sexual maturity, faster body size increase, or altered ossification timing, forelimb elements may develop differently relative to hindlimbs than in ancestral forms. In birds and their close relatives, developmental plasticity along the wing-leg axis has repeatedly produced varied locomotor profiles across clades.
A third limitation of viewing early birds through modern adult birds is ignoring ontogeny. Juveniles and subadults often face different ecological pressures than adults, and shifts in developmental schedules can carry adult locomotor consequences—including reduced or lost flight capacity.
Causal Chains That Sensational Coverage Misses
Standard news coverage tends to list traits in isolation: small wings here, thick bones there, unexpected anywhere. Real biological systems run on causal chains where one shift triggers downstream constraints.
Trace a plausible causal sequence in a localized, resource-rich habitat. First, abundant ground or shoreline food lowers the search cost of staying off the wing. Second, reduced selection for long-distance aerial commuting allows subtle shifts in wing-to-leg proportions or flight-muscle investment. Third, altered body mass and wing loading change takeoff mechanics, making frequent flight costlier relative to walking, running, or swimming. Fourth, once flight becomes energetically expensive to initiate, selection increasingly refines non-aerial locomotion, reinforcing the shift away from habitual flight.
Notice what happens at the end of that chain. The organism is not "failing to evolve." It is optimizing for a specific fitness landscape where aerial flight no longer pays its full metabolic toll.
Consider a conceptual example from modern and deep-time ecology: an island or isolated habitat where terrestrial predators are scarce and ground foraging is lucrative. Over generations, lineages that trim flight investment gain energetic efficiency. Yet if a new ground predator arrives or food patches scatter across water barriers, that same specialization becomes a vulnerability. High specialization increases efficiency within a narrow band of conditions while narrowing resilience when conditions shift.
Operationalizing This Framework for Research and Analysis
Whether you are evaluating a new fossil paper, editing science coverage, or building an analytical model of trait evolution, a disciplined workflow prevents sloppy conclusions.
- Audit the claim against the evidence: Separate the anatomical description and geological context from the behavioral or evolutionary headline. Check whether flightlessness is demonstrated by clear biomechanical indicators or inferred from partial remains.
- Map the phylogenetic context: Determine where the taxon sits relative to close relatives. Repeated appearance of a trait across branches points toward convergent responses to similar pressures rather than a single freak accident.
- Evaluate trade-offs across systems: Look at forelimbs, hindlimbs, torso proportions, and habitat indicators together. A change in one locomotor module almost always shifts loads or energy budgets elsewhere.
- Separate mechanism from narrative: Ask what selection pressure, developmental shift, or ecological constraint could drive the trait, and state clearly which parts remain unproven.
Where This Analytical Model Hits Limits
No analytical framework solves every paleontological puzzle. Fossilization is an incomplete filter, and many Mesozoic environments lack preservation altogether. Biomechanical estimates from fossil skeletons depend on assumptions about soft tissue volume, muscle attachment geometry, and bone properties that cannot be measured directly from rock alone.
Furthermore, correlation in the fossil record does not automatically prove causation. Two traits—such as reduced wing length and a wetland deposit—may co-occur because of a shared third factor, such as body size or evolutionary history, rather than direct cause and effect. Analysts who treat a framework as an infallible truth-machine will overfit sparse data.
Strategic Play for Science Communicators and Analysts
Stop framing evolutionary divergence as a contest between "winners" that fly and "losers" that do not. Build your coverage and analysis around locomotor trade-offs and environmental fit, treating every flightless early avialan as a data point on how natural selection balances energy budgets, habitat structure, and developmental pathways. When you replace sensationalist shock with clear causal mechanics, your analysis stays accurate even as new fossils refine the family tree.


